Synaptic plasticity is the nervous system’s lifelong ability to strengthen, weaken, add or remove connections between neurons in response to experience. It is widely regarded as the cellular basis of learning and memory.
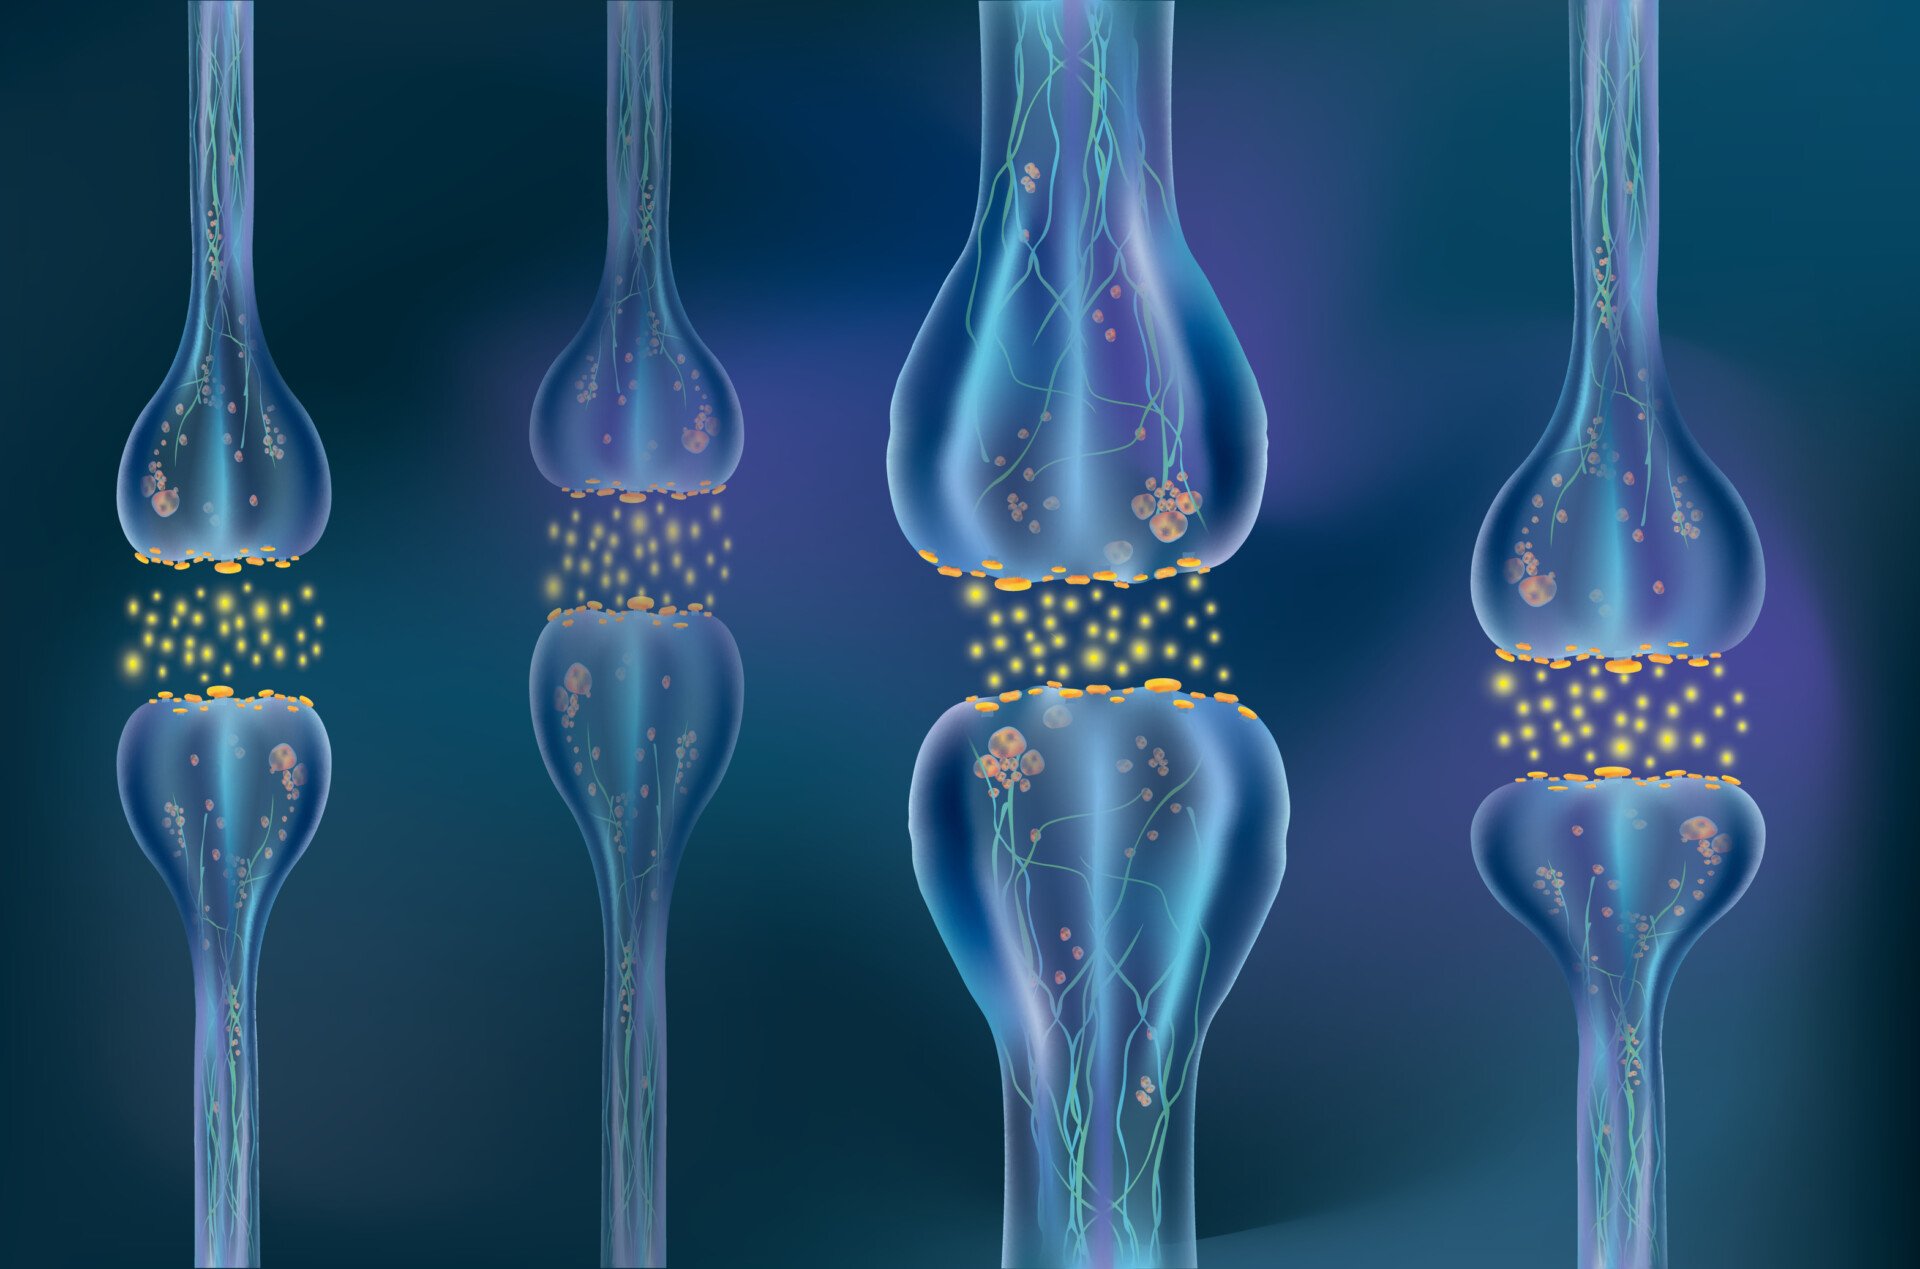
At its core, it involves alterations in the strength and structure of connections, known as synapses, between neurons.
This dynamic process includes strengthening and weakening existing synapses, creating new ones, and pruning those no longer needed.
New neurons arise through a separate process, neurogenesis. Synaptic plasticity is the smallest-scale form of neuroplasticity, working at the level of individual synapses.
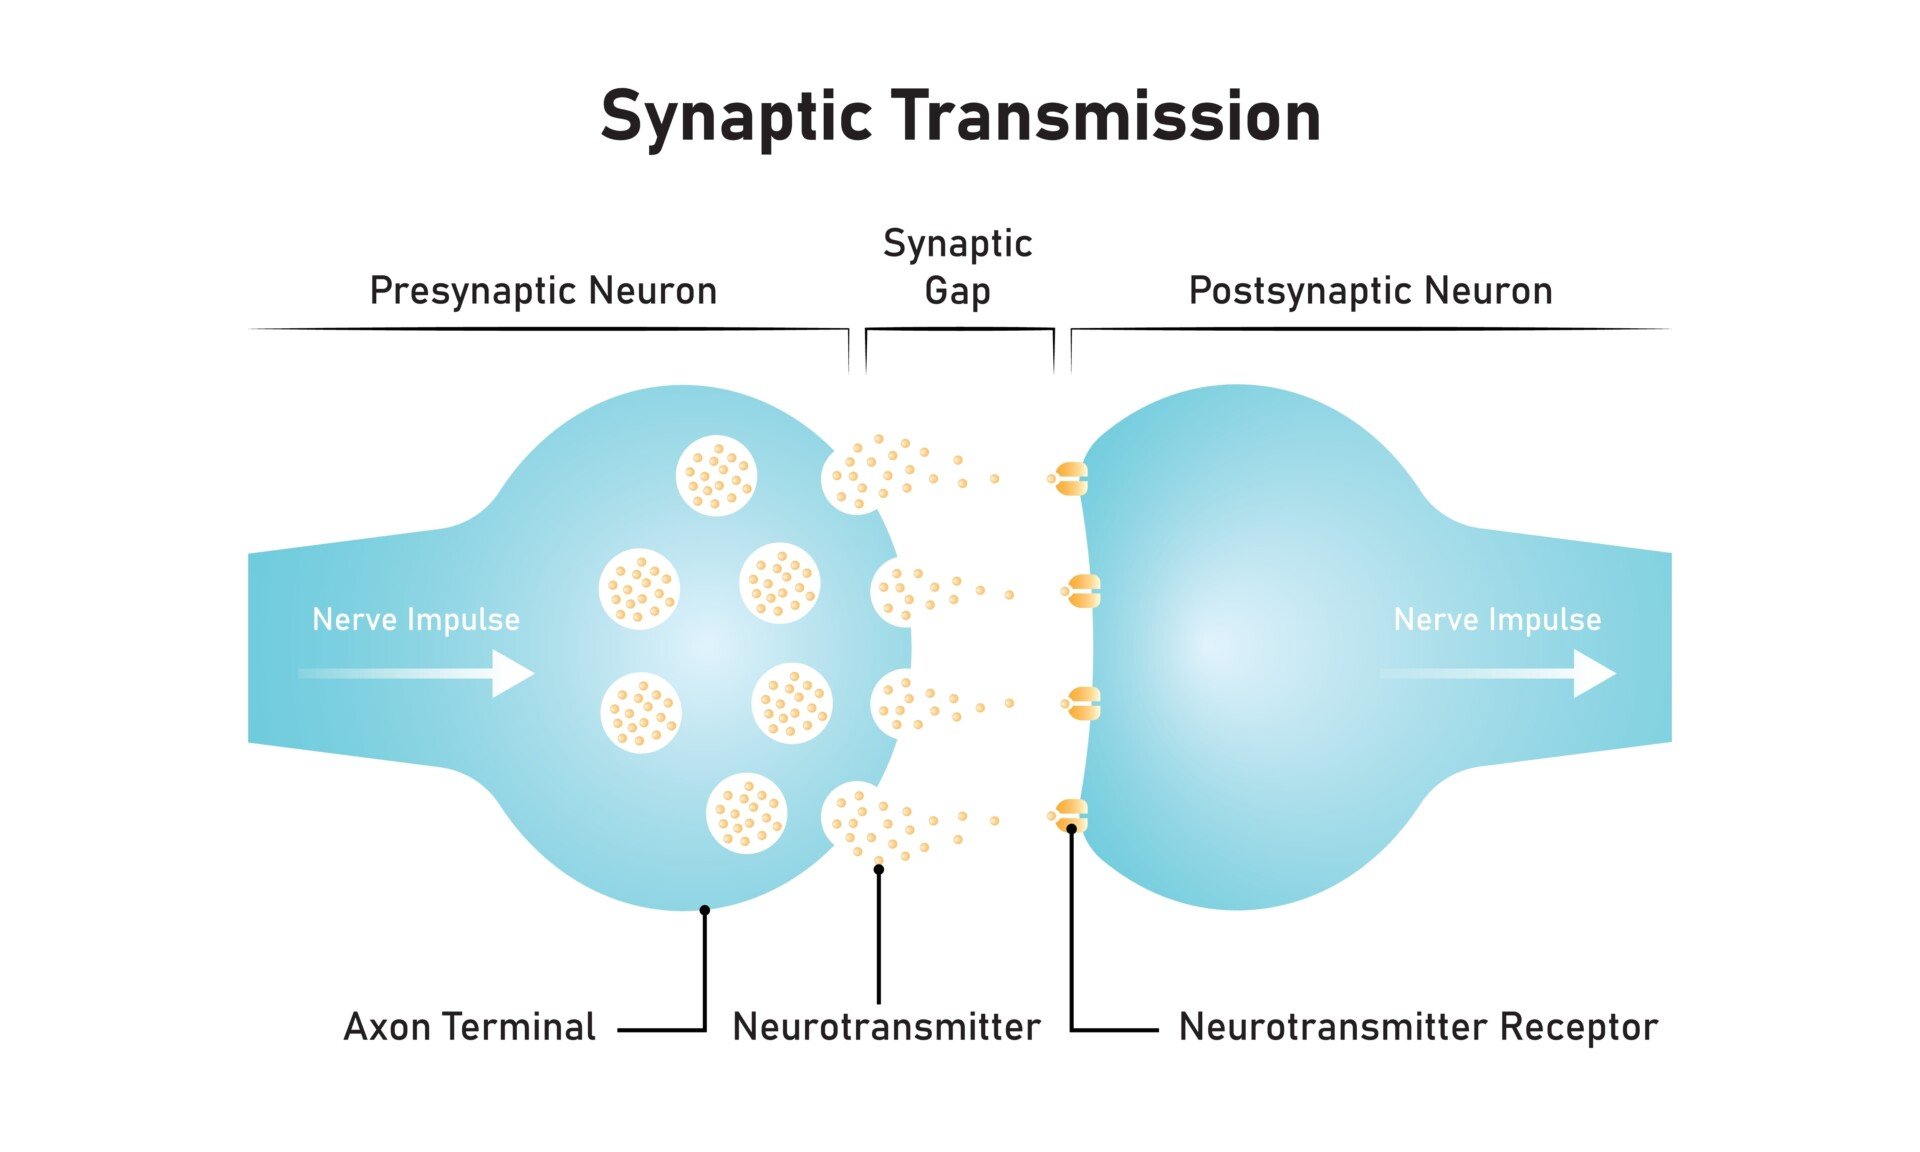
Neurotransmitters, the chemical messengers released across the synaptic gap, are crucial for these changes. They help trigger long-term potentiation (LTP), a lasting increase in the strength of a synapse.
This property underpins brain function, enabling learning and adaptation.
When you learn a new skill like playing the violin, the brain areas for finger movements physically change and grow. That is brain adaptation in action.
Similarly, forming new habits involves the continuous reshaping of neural circuits through synaptic plasticity.
Types of synaptic plasticity
There are two main types of synaptic plasticity based on how long the changes last:
Short-term synaptic plasticity
This involves quick adjustments that last from milliseconds to a few minutes. These often affect how much chemical message (neurotransmitter) is released from one neuron to another.
For example, a rapid burst of activity might temporarily increase (facilitation) or decrease (depression) the communication strength at a synapse.
These changes fade quickly. They are thought to support very short-term information processing rather than durable memory. Habituation of a sea slug’s withdrawal reflex is a classic example (see Kandel’s Aplysia research, below).
Long-term synaptic plasticity
These changes are longer-lasting, persisting for days, weeks, or even longer. There are two important forms:
- Long-Term Potentiation (LTP): This is a long-lasting increase in synaptic strength, first demonstrated in 1973 (Bliss & Lømo, 1973). It usually involves adding AMPA receptors (which receive signals) after special receptors called NMDA receptors are activated, so the receiving neuron fires more easily.
- Long-Term Depression (LTD): This is the opposite of LTP: a long-lasting decrease in synaptic strength. It happens when AMPA receptors are removed or dendritic spines (tiny parts of the neuron receiving signals) shrink or disappear, so the neuron is less easily activated.
Together, LTP and LTD help balance and fine-tune connections between neurons, shaping how the brain develops, learns, and remembers.
Bliss and Lømo (1973): The Discovery of LTP
Bliss and Lømo (1973) gave the first direct demonstration of a lasting, activity-dependent change in the mammalian brain. Their rabbit experiment remains the foundation of the field.
- Aim: To test whether brief, high-frequency stimulation of a pathway into the hippocampus could produce a durable increase in synaptic strength.
- Method: In anaesthetised rabbits, they stimulated the perforant path and recorded from the dentate gyrus. After a stable baseline, they applied short high-frequency trains (tetani), then resumed test stimulation.
- Results: The synaptic response grew larger and more cells fired. The enhancement lasted for hours in acute preparations and for days or weeks in chronically implanted animals.
- Conclusion: Synapses in the mammalian brain can undergo a lasting, activity-dependent increase in strength, soon named long-term potentiation (LTP).
That persistence made LTP the leading candidate mechanism for memory storage. It has held that status ever since.
Mechanisms of Synaptic Plasticity
Synaptic plasticity involves biochemical and structural changes at the neuronal level:
- Chemical Signals and Receptors: NMDA receptors are glutamate-gated channels that open only when a neuron is already active. Calcium entry then adds or sensitizes AMPA receptors (LTP) or removes or desensitizes them (LTD).
- Structural Changes: Synapses physically remodel through dendritic spine growth or shrinkage. LTP can create new connections, while LTD eliminates or weakens existing ones.
- Protein Synthesis: Long-lasting plasticity requires gene activation and new proteins (e.g., brain-derived neurotrophic factor [BDNF]), enhancing synaptic health and supporting sustained changes.
- Timing and Activity Patterns: Spike-timing-dependent plasticity (STDP) is a rule where millisecond firing order sets the direction of change. Presynaptic (sending) firing just before postsynaptic (receiving) activity promotes LTP, while reversed timing promotes LTD (Markram et al., 1997; Bi & Poo, 1998).
- Homeostatic Plasticity: Neurons globally scale their synaptic strengths up or down to keep activity stable, maintaining neural balance (Turrigiano & Nelson, 2004).
Hebb’s Rule and the NMDA Receptor
Donald Hebb (1949) proposed the principle behind most plasticity research. As Hebb explained in The Organization of Behavior:
“When an axon of cell A is near enough to excite a cell B and repeatedly or persistently takes part in firing it, some growth process or metabolic change takes place in one or both cells such that A’s efficiency, as one of the cells firing B, is increased.”
This is popularly summarised as “cells that fire together, wire together.”
It turned an old psychological idea, association by contiguity, into a physiological prediction that could be tested at a single synapse.
The NMDA receptor is the molecular implementation of this rule. It acts as a coincidence detector.
At resting potential, a magnesium ion plugs its channel. It opens only when glutamate (released by the sending neuron) is present and the receiving neuron is already depolarised.
When the channel opens, calcium flows in. A large, rapid rise activates enzymes such as CaMKII, which drive more AMPA receptors into the membrane (LTP). A smaller, prolonged rise activates enzymes that remove AMPA receptors instead (LTD; Malenka & Nicoll, 1999).
This single mechanism explains three defining properties of LTP:
- Input specificity: Only synapses active during stimulation are strengthened, so one neuron can store many independent memories.
- Cooperativity: Enough inputs must fire together to depolarise the cell and expel the magnesium block.
- Associativity: A weak input is strengthened if it is active alongside a strong one, a cellular analogue of associative learning.
Relevance to psychology
Synaptic plasticity is crucial for psychology because it explains how our brains literally change to support our thoughts, feelings, and behaviours.
Learning and Memory
This brain plasticity is the physical basis for all learning and memory formation. When we learn new information, like facts for a test, our brain’s synapses are strengthened.
LTP is believed to be a key process in forming memories. LTD helps refine existing memories by weakening unneeded connections.
Education offers a clear example. Roediger and Karpicke (2006) found that students tested on studied material remembered substantially more a week later than students who re-read it. Yet re-reading had felt more effective.
A Hebbian account explains why. Successful retrieval reactivates and strengthens the synapses that store the memory, whereas passive re-reading provides weaker input.
Classical conditioning, where an association is learned between two stimuli (like Pavlov’s dogs), also relies on these plastic changes.
Kandel’s Aplysia Research: From Synapse to Gene
Eric Kandel and colleagues traced simple learning to individual synapses in the sea slug Aplysia. Its small number of large, identifiable neurons made this possible. The work was recognised with a Nobel Prize.
Habituation and Sensitisation
Castellucci et al. (1970) studied two simple forms of learning in the slug’s gill-withdrawal reflex:
- Habituation: The reflex fades with repeated harmless touch, reflecting a drop in neurotransmitter release from the sensory neuron.
- Sensitisation: The reflex strengthens after a noxious stimulus, because serotonin increases that release.
Changes like these modify existing proteins and need no new protein synthesis. Short-term memory is stored in pre-existing connections.
CREB and Long-Term Memory
Dash et al. (1990) asked what makes a change last. They injected short DNA fragments into the nucleus of sensory neurons. The fragments act as decoys that trap CREB, a transcription factor that switches genes on.
Long-term facilitation vanished a day later, while short-term facilitation was untouched. Long-term memory therefore needs gene transcription and new proteins.
Kandel (2001) drew these threads together. Repeated training moves enzymes to the nucleus, where CREB switches on genes that stabilise and grow new synaptic connections. Early and late LTP in the hippocampus follow the same pattern: a fast phase that needs no new proteins, then a slower, gene-dependent structural phase.
Brain Development and Neural Reorganization
Synaptic plasticity underlies brain development and neural reorganization throughout our lives.
In early life, there’s a rapid “blooming” of neural connections. Activity-dependent “pruning” then removes little-used connections, an LTD-like process, while active ones are consolidated. This sculpts more efficient circuits for complex skills, and the process continues into adolescence.
This adaptation allows the brain to respond to and be shaped by its environment.
Recovery and Adaptation
Plasticity also supports recovery and adaptation, especially after brain injury. The brain can reorganise itself after damage, and this neuroplasticity is why people can regain functions after a stroke.
Rehabilitation harnesses this plasticity. Kleim and Jones (2008) summarised the evidence as principles of experience-dependent plasticity:
- Use-Dependence: Practice, not passive stimulation, drives reorganisation.
- Specificity: The behaviour practised is the one that reorganises.
- Repetition and Intensity: Both matter for lasting change.
- Reversibility: Unused circuits can lose cortical territory (“use it or lose it”), while practised ones expand.
Constraint-induced movement therapy applies these principles. It restrains a stroke survivor’s unaffected limb, forcing repeated, intensive use of the affected one. Taub and Uswatte (2006) reported lasting motor gains and expansion of the cortical representation of the trained limb.
However, when this process goes wrong, it can contribute to neuropsychiatric conditions like schizophrenia, where impaired plasticity is observed.
Factors influencing synaptic plasticity
Synaptic plasticity is influenced by many factors:
- Age and Developmental Stage: While the brain is most plastic when we are young, it continues to change and adapt throughout our entire lives. For instance, certain cognitive abilities and how the brain processes information can differ between adolescents and adults, reflecting ongoing development.
- Sleep Quality and Cognitive Function: Getting enough good quality sleep is crucial for brain health. Insufficient sleep or sleep disorders can significantly impair a wide range of cognitive functions, including memory and attention. Poor sleep can even reduce hippocampal synaptic plasticity, which is vital for memory formation.
- Stress and Mental Health: Chronic stress and past traumatic experiences, especially during childhood, can negatively impact brain circuits and reduce the brain’s ability to adapt, potentially increasing vulnerability to conditions like depression and schizophrenia.
- Exercise and Nutrition: Physical exercise promotes neuroplasticity, boosting cognitive function and stimulating growth factors like BDNF that are involved in synaptic regulation, learning, and memory. Proper nutrition is also essential for healthy brain development, and poor nutrition impairs cognitive abilities.
Disorders linked to synaptic plasticity
Alzheimer’s disease
This neurodegenerative condition is characterized by progressive cognitive decline, especially memory loss.
Alzheimer’s may begin as a synaptic failure. Selkoe (2002) argued that soluble amyloid-β oligomers impair NMDA-receptor-dependent LTP and drive synapse loss. This happens well before the plaques and cell death that define the disease, which helps explain why memory problems appear first.
In mouse models of early Alzheimer’s, memories that seemed lost were recovered by reactivating the neurons that stored them (Roy et al., 2016). Memory loss may reflect blocked access, not erasure.
Schizophrenia
This disorder involves symptoms like disorganized thinking and behaviour, as well as significant cognitive deficits. Disrupted synaptic plasticity is implicated in these deficits.
Individuals often show reduced connections (spine density) and problems with how their brain cells communicate, impacting their ability to process information, learn, and remember. Researchers implicate NMDA-receptor hypofunction, meaning underactive NMDA receptors, in these changes. That matters because NMDA receptors are the coincidence detectors that trigger LTP and LTD.
Addiction
Drugs of abuse hijack the same synaptic machinery that stores adaptive memories. Kauer and Malenka (2007) reviewed the evidence. One exposure to cocaine, amphetamine or opioids can strengthen excitatory synapses onto dopamine neurons in the ventral tegmental area.
Repeated exposure drives further, more persistent plasticity in projections to the nucleus accumbens and prefrontal cortex.
On this view, addiction is a form of maladaptive memory. Cues linked to the drug become powerful triggers for craving because the synapses connecting cue and reward circuitry have been potentiated. That is why relapse can occur long after the drug’s direct effects have worn off.
Depression and anxiety disorders
Impaired plasticity is not the whole story. But these conditions can involve difficulties in the brain’s ability to adapt and learn new, healthier responses.
Chronic stress and trauma can negatively affect brain circuits. This reduces their capacity for adaptive change.
Individuals often experience cognitive impairment, such as problems with attention, processing information, and memory. This can reflect a struggle to “unlearn” unhelpful thought patterns or behaviours.
Critical Evaluation
The framework’s main strength is convergence. Two lines of evidence reach the same principle independently: activity-dependent, calcium-triggered change in synaptic strength.
One line is rabbit hippocampal LTP (Bliss & Lømo, 1973). The other is sea slug molecular biology (Castellucci et al., 1970; Kandel, 2001). The framework also yields practical levers in rehabilitation, education and addiction research.
The Synaptic Plasticity and Memory Hypothesis
The synaptic plasticity and memory (SPM) hypothesis holds that activity-dependent plasticity is both necessary and sufficient for storing memories. Martin et al. (2000) made it testable with four criteria:
- Detectability: If a memory forms, a change in synaptic strength should be detectable in the relevant circuit.
- Mimicry: Artificially creating the pattern of synaptic weights should produce an apparent, false memory.
- Anterograde alteration: Blocking or saturating plasticity before learning should prevent new memories forming.
- Retrograde alteration: Erasing the plastic change after learning should abolish the memory it stored.
Two classic experiments tested the first and third criteria. Morris et al. (1986) infused rats with AP5, a drug that blocks NMDA receptors and prevents LTP. The rats failed to learn a hidden platform’s location in a water maze but performed normally when the platform was visible.
Whitlock et al. (2006) recorded from hippocampal area CA1 as rats learned an avoidance task in a single session. Learning itself strengthened AMPA-receptor-mediated transmission at a subset of synapses.
It also used up capacity for further electrically induced LTP, because both share a mechanism. That was direct evidence that learning induces LTP.
Rival and Complementary Models
The Hebbian LTP account is dominant, but three alternative models temper how it should be read:
- Homeostatic Plasticity: Hebbian strengthening alone would spiral into runaway excitation. Turrigiano and Nelson (2004) described synaptic scaling, which adjusts all of a neuron’s synapses over hours to days to restore stable firing.
- BCM Theory: Bienenstock et al. (1982) proposed that the activity threshold for potentiation slides up after high activity and down after low activity. Calcium-dependent signalling (Malenka & Nicoll, 1999) offers a plausible biological basis.
- Complementary Learning Systems: McClelland et al. (1995) argued that the hippocampus encodes new experience quickly, then slowly trains distributed representations in the neocortex. Memory may therefore migrate rather than stay in fixed hippocampal synapses.
These models are best read as complements, not rivals. Homeostatic plasticity stabilises a Hebbian network. BCM theory explains why a threshold should slide, while NMDA-receptor calcium signalling explains how.
Limitations of the Evidence
Several limits remain:
- Animal Models: Much direct evidence comes from anaesthetised rabbits, cultured neurons and a sea slug’s reflex, so the leap to human memory is indirect.
- Rodent-Only Causal Tests: Experiments that manipulate memory directly are confined to animals. Human evidence is weaker, mostly correlational or lesion-based.
- Memory Is Not Just a Strong Synapse: Engram research (below) suggests strength governs how accessible a memory is. The information itself may reside in the pattern of connectivity.
- Adaptive and Maladaptive Learning: The same machinery stores useful memories and drug-associated cues, so “more plasticity” is not always better.
- Unjoined Levels: How brief synaptic changes become lifelong memories, and how hippocampal traces move to cortex, remain open questions.
None of these limits undermines the core finding. They show that synaptic plasticity is necessary for memory but not the whole story.
Contemporary Research
Optogenetics uses light to switch genetically tagged neurons on or off. It now lets researchers label the neurons active during an experience, the putative memory engram, and manipulate them. It tests the hypothesis’s hardest criteria: mimicry and retrograde alteration.
From Sufficiency to Synaptic Weight
Liu et al. (2012) tagged dentate-gyrus neurons active during fear conditioning with a light-sensitive channel. Reactivating just those cells with light in a neutral context made the animals freeze, as if recalling the fear.
Reactivating an engram was therefore sufficient to trigger recall.
Nabavi et al. (2014) then conditioned an association onto optically stimulated amygdala inputs. Low-frequency (LTD-inducing) stimulation inactivated the memory, and high-frequency (LTP-inducing) stimulation reinstated it.
The memory tracked the direction of synaptic change.
Memory Without Synaptic Strengthening
Ryan et al. (2015) induced retrograde amnesia in animals by giving anisomycin, a protein-synthesis inhibitor, shortly after fear conditioning. The animals did not recall the context naturally.
Their engram cells also lacked the usual rise in synaptic strength and spine density.
Yet reactivating the engram with light still produced full recall. The memory had survived. Synaptic strengthening may be needed for natural retrieval rather than for storage itself.
Restoring Memories in an Alzheimer’s Model
Roy et al. (2016) tested the same idea in a disease model.
- Aim: To test whether memory loss in early Alzheimer’s reflects failed storage or failed access to an intact engram.
- Method: Mice carrying an early-Alzheimer’s-like mutation forget fear memories quickly. Engram cells in the dentate gyrus were labelled during learning, then reactivated with light once natural recall had failed.
- Results: Engram cells had fewer spines and weaker synapses, and natural recall failed. Yet light reactivation restored freezing to healthy-control levels.
- Conclusion: Early memory loss can reflect blocked retrieval from a weakened but intact engram, not erased storage.
Repeated stimulation over several days even partially restored spine density and some natural recall. If memories are unreachable rather than gone, restoring access becomes a plausible therapeutic goal.
Potentiation as a Cause
Cardozo et al. (2025) moved from whole cells to synapses. In the mouse amygdala, they measured the AMPAR/NMDAR current ratio, an index of how strongly a synapse is potentiated, at inputs onto shock-responsive neurons. Fear conditioning raised the ratio only at these synapses, and extinction reversed it.
Inducing the same potentiation optogenetically, with no shock at all, was enough to create a fear association to a neutral context. Potentiation was necessary and sufficient.
Weighing the Evidence
Together, these studies give the strongest evidence yet for the SPM hypothesis. Memories can be found, activated, erased and reinstated by targeting specific neurons and synapses.
Yet they also refine it. Synaptic strength appears to govern how accessible a memory is, while its identity may lie in the connectivity among its cells.
Ways to Enhance Synaptic Plasticity
Practical strategies to improve synaptic plasticity include:
- Lifelong Learning: Regular mental stimulation through learning languages, skills, or engaging activities promotes synaptic growth.
- Physical Exercise: Aerobic exercise increases BDNF levels, enhancing cognitive health and plasticity.
- Quality Sleep: Sufficient sleep consolidates memories, resets synaptic strengths, and supports learning.
- Stress Management: Mindfulness, therapy, and relaxation techniques reduce stress-induced impairments in plasticity.
- Healthy Diet: Nutrient-rich diets (e.g., Mediterranean diet) support neuronal health and cognitive aging.
- Social Interaction: Active social engagement stimulates diverse neural networks, enhancing plasticity.
- Cognitive Training: Targeted cognitive exercises can enhance specific skills, promoting corresponding neural changes.
Key Takeaways
- Definition: Synaptic plasticity is the ability of synapses to strengthen or weaken with activity. It is widely regarded as the cellular basis of learning and memory.
- LTP and LTD: Long-term potentiation strengthens a synapse for hours or longer, while long-term depression weakens it. Together they balance and refine connections.
- Hebb’s Rule: Cells that fire together wire together. NMDA receptors detect this coincident activity and trigger the change.
- Lasting Memory: Lasting change needs gene expression and new proteins, which stabilise and grow synapses.
- Evidence: Blocking LTP impairs learning in rats, and engram studies show memories can be reactivated by targeting specific neurons.
- Limits: Causal evidence comes mostly from animals, and a memory is not simply a strengthened synapse.
- Modifiers: Sleep, stress, exercise and age shape plasticity, which continues throughout life.
References
Bi, G.-Q., & Poo, M.-M. (1998). Synaptic modifications in cultured hippocampal neurons: Dependence on spike timing, synaptic strength, and postsynaptic cell type. The Journal of Neuroscience, 18(24), 10464–10472. https://doi.org/10.1523/JNEUROSCI.18-24-10464.1998
Bienenstock, E. L., Cooper, L. N., & Munro, P. W. (1982). Theory for the development of neuron selectivity: Orientation specificity and binocular interaction in visual cortex. The Journal of Neuroscience, 2(1), 32–48. https://doi.org/10.1523/JNEUROSCI.02-01-00032.1982
Bliss, T. V. P., & Lømo, T. (1973). Long-lasting potentiation of synaptic transmission in the dentate area of the anaesthetized rabbit following stimulation of the perforant path. The Journal of Physiology, 232(2), 331–356. https://doi.org/10.1113/jphysiol.1973.sp010273
Cardozo, L. M., de Sousa, A. F., Dillingham, B. C., Dang, W., Job, N., Yoo, E. J., Ranamukhaarachchi, S. K., Yuan, Q., & Mayford, M. (2025). Synaptic potentiation of engram cells is necessary and sufficient for context fear memory. Communications Biology, 8, Article 862. https://doi.org/10.1038/s42003-025-08140-6
Castellucci, V., Pinsker, H., Kupfermann, I., & Kandel, E. R. (1970). Neuronal mechanisms of habituation and dishabituation of the gill-withdrawal reflex in Aplysia. Science, 167(3926), 1745–1748. https://doi.org/10.1126/science.167.3926.1745
Dash, P. K., Hochner, B., & Kandel, E. R. (1990). Injection of the cAMP-responsive element into the nucleus of Aplysia sensory neurons blocks long-term facilitation. Nature, 345(6277), 718–721. https://doi.org/10.1038/345718a0
Hebb, D. O. (1949). The organization of behavior: A neuropsychological theory. Wiley.
Kandel, E. R. (2001). The molecular biology of memory storage: A dialogue between genes and synapses. Science, 294(5544), 1030–1038. https://doi.org/10.1126/science.1067020
Kauer, J. A., & Malenka, R. C. (2007). Synaptic plasticity and addiction. Nature Reviews Neuroscience, 8(11), 844–858. https://doi.org/10.1038/nrn2234
Kleim, J. A., & Jones, T. A. (2008). Principles of experience-dependent neural plasticity: Implications for rehabilitation after brain damage. Journal of Speech, Language, and Hearing Research, 51(1), S225–S239. https://doi.org/10.1044/1092-4388(2008/018)
Liu, X., Ramirez, S., Pang, P. T., Puryear, C. B., Govindarajan, A., Deisseroth, K., & Tonegawa, S. (2012). Optogenetic stimulation of a hippocampal engram activates fear memory recall. Nature, 484(7394), 381–385. https://doi.org/10.1038/nature11028
Malenka, R. C., & Nicoll, R. A. (1999). Long-term potentiation: A decade of progress? Science, 285(5435), 1870–1874. https://doi.org/10.1126/science.285.5435.1870
Markram, H., Lübke, J., Frotscher, M., & Sakmann, B. (1997). Regulation of synaptic efficacy by coincidence of postsynaptic APs and EPSPs. Science, 275(5297), 213–215. https://doi.org/10.1126/science.275.5297.213
Martin, S. J., Grimwood, P. D., & Morris, R. G. M. (2000). Synaptic plasticity and memory: An evaluation of the hypothesis. Annual Review of Neuroscience, 23(1), 649–711. https://doi.org/10.1146/annurev.neuro.23.1.649
McClelland, J. L., McNaughton, B. L., & O’Reilly, R. C. (1995). Why there are complementary learning systems in the hippocampus and neocortex: Insights from the successes and failures of connectionist models of learning and memory. Psychological Review, 102(3), 419–457. https://doi.org/10.1037/0033-295X.102.3.419
Morris, R. G. M., Anderson, E., Lynch, G. S., & Baudry, M. (1986). Selective impairment of learning and blockade of long-term potentiation by an N-methyl-D-aspartate receptor antagonist, AP5. Nature, 319(6056), 774–776. https://doi.org/10.1038/319774a0
Nabavi, S., Fox, R., Proulx, C. D., Lin, J. Y., Tsien, R. Y., & Malinow, R. (2014). Engineering a memory with LTD and LTP. Nature, 511(7509), 348–352. https://doi.org/10.1038/nature13294
Roediger, H. L., & Karpicke, J. D. (2006). Test-enhanced learning: Taking memory tests improves long-term retention. Psychological Science, 17(3), 249–255. https://doi.org/10.1111/j.1467-9280.2006.01693.x
Roy, D. S., Arons, A., Mitchell, T. I., Pignatelli, M., Ryan, T. J., & Tonegawa, S. (2016). Memory retrieval by activating engram cells in mouse models of early Alzheimer’s disease. Nature, 531(7595), 508–512. https://doi.org/10.1038/nature17172
Ryan, T. J., Roy, D. S., Pignatelli, M., Arons, A. L., & Tonegawa, S. (2015). Engram cells retain memory under retrograde amnesia. Science, 348(6238), 1007–1013. https://doi.org/10.1126/science.aaa5542
Selkoe, D. J. (2002). Alzheimer’s disease is a synaptic failure. Science, 298(5594), 789–791. https://doi.org/10.1126/science.1074069
Taub, E., & Uswatte, G. (2006). Constraint-induced movement therapy: Answers and questions after two decades of research. NeuroRehabilitation, 21(2), 93–95. https://doi.org/10.3233/NRE-2006-21201
Turrigiano, G. G., & Nelson, S. B. (2004). Homeostatic plasticity in the developing nervous system. Nature Reviews Neuroscience, 5(2), 97–107. https://doi.org/10.1038/nrn1327
Whitlock, J. R., Heynen, A. J., Hussain Shuler, M. G., & Bear, M. F. (2006). Learning induces long-term potentiation in the hippocampus. Science, 313(5790), 1093–1097. https://doi.org/10.1126/science.1128134